Showing posts with label race. Show all posts

Monday, June 30, 2025

Razib Khan on Denisovans

Razib Khan does a good job of summing up some of the things that we've learned in recent years about Denisovans, an archaic hominin clade.

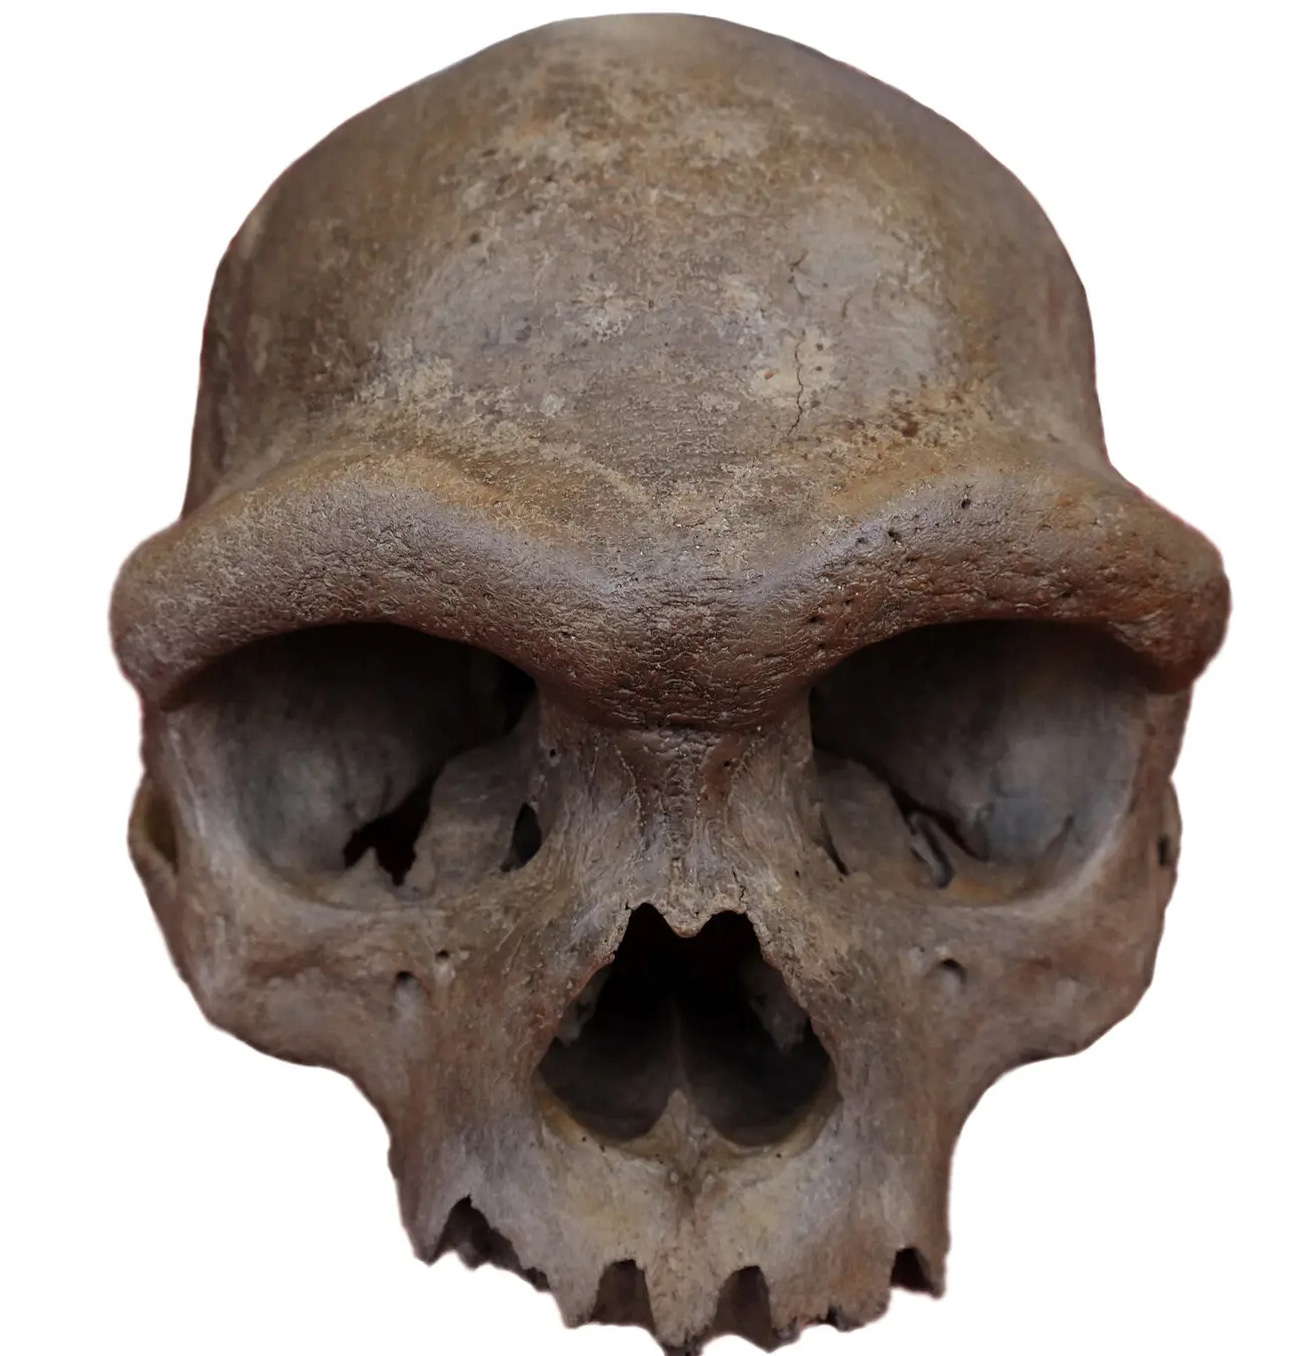
[I]n June 2025, Chinese paleogeneticist Qiaomei Fu published data finally connecting specific fossil remains to Denisovans, utilizing both mtDNA and protein sequencing methods. And so now we know that Denisovans and Homo longi, are one and the same. A rather well preserved fossil from Harbin, China, a nearly complete skull, first identified as a new species in a 2021 publication, and colloquially dubbed Dragon Man, turns out to have DNA that we can now see neatly matches the sequences extracted from Denisova cave. For fifteen years, the label Denisovan only applied in a genomic context. No longer. Denisovan physical remains were in fact in plain sight all along.

This is not entirely a surprise. Some geneticists and paleoanthropologists have long assumed that many among the wealth of the fossils languishing yet to be identified, catalogued or named in East Asian collections today were Denisovans (I said as much in a podcast with Vagheesh Narasimhan of UT Austin, when H. longi was announced four years ago). Also, since 2010, we have established that Denisovans are the ancestors of more than Papuans and other Australasians. The Negrito peoples of the Philippines have a substantial contribution from Denisovans, the same as their Papuan neighbors from New Guinea to the south. But when you set aside their majority Austronesian ancestry (a much more recent overlay), it appears their forager ancestors (today some 35% of their ancestry) carried even more Denisovan ancestry than Papuans, on the order of 7-8%. It is also clear that low, but detectable, levels of Denisovan ancestry appear today in populations across South, East and Southeast Asia, at fractions of 0.1-0.3%.


Partial skull of Homo longi, AKA a Denisovan

The attested presence of Denisovan ancestry across a vast triangle stretching from Pakistan to Japan to Australia argues that they were present across vast territories. Deeper analysis of the Denisovan fragments in the genomes of Asians, Melanesians and Australians suggest at minimum two admixture events with two very distinct Denisovan populations. One population is clearly related to the genomes we have from Denisova cave. These northern Denisovans mixed with the ancestors of modern East Asians. But the Denisovan ancestry in South and Southeast Asians, as well as in Melanesians and Australians, is clearly from a population with a distinct ancestry; likely one that split off from the northern subspecies as long as more than 350,000 years ago. And the plot thickens, because tentative evidence gleaned from comparing the segments carried by these populations with southern Denisovan ancestry suggests distinct admixtures here as well; one in South Asians, another in Southeast Asians (a common one with Melanesians and Australians), and perhaps even one or two further ones in the outer reaches of prehistoric Sundaland and Sahul.

Friday, February 28, 2025

The Intra-African Slave Trade And Its Consequences

Contrary to some "Afro-Centric" educators, Egypt is darker skinned and has more sub-Saharan ancestry (as confirmed by modern and ancient DNA) now than it did in the classical era and in earlier times.

What happened?


A lot of sub-Saharan Africans were forced into slavery and delivered to the Middle East and North Africa (including Egypt) during the Middle Ages.

Monday, November 1, 2021

The Tarim Mummies Were Not Migrants From Steppe; Horses Did Not Drive Early Indo-European Expansion

A pair of late October 2021 papers have upset conventional paradigms about some of the details about the early spread of the Indo-Europeans, although most of the narrative remains intact.

Early Tarim Mummies Weren't From The Steppe

The Tarim Mummies ca. 2000 BCE were Paleo-Siberians who adopted herding and farming practices by cultural diffusion from neighboring populations.

Populations descended from the presumptively Indo-European Afanasievo people brought the Tocharian language eventually spoken in the Tarim Basin, which is a basal Indo-European language. They settled in the arid mountain ringed basin to the immediate North of the Tarim Basin, called Dzungaria ca. 3000 BCE (splitting off from the main steppe Indo-European population at that time). These people migrated to the Tarim basin, bringing their language with them, starting more than a thousand years later.

Indo-Iranian people came and admixed next which is why the Tarim basin people looked a lot like white people in art from ca. 500-1000 CE.


The paper that reported on the data from the famous “Tarim Mummies” is out. . . . it now looks that the Tarim populations from 4,000 years ago are among the last people who were mostly “Ancestral North Eurasian” (ANE), and, they had no connection to populations in Europe. . . . 
the earlier remains from Dzungaria are mostly descended from Afanasievo populations with a minority of ANE ancestry. The authors conclude, correctly I think, that this points to the likely origins of the Tocharian languages from the Afanasievo, and the possibility (I bet) that the ancient Yamnaya language was similar to that of the Tocharians. The fact that the Tarim people seem to have been mostly very distant branches of [Y-DNA haplogroup] R1b illustrates the origin of the R lineage deep in Siberia during the Pleistocene. R and Q are clearly from the Paleo-Siberians. . . . 
These results in this paper show that the core population 4,000 years ago in the region of the Tarim that was later home to the Tocharians was inhabited by an ANE/Paleo-Siberian population, with a minority component of ancestry derived from northern East Asians. This ancestry dates to the early Holocene, 10,000 years ago. The later Tocharians probably absorbed these people, but I believe they were a mix of post-Afanasievo populations and Iranians. The former gave the Tocharians their unique and very basal Indo-European language, and the latter were responsible for “European” physical features so noted by the Han Chinese chroniclers in the 1st millennium A.D.

Note: the ANE are closer to West Eurasians than East Eurasians, but they are very distantly related to the former. Their ancestors seem to have diverged from European and West Asian hunter-gatherers 35,000 to 40,000 years ago.

From Razib Khan at Gene Expression. 

Bernard's Blog explains (translation from French via Google):

[A]ncient individuals of Dzungaria have between 50 and 70% of Afanasievo ancestry, between 19 and 36% of an ANE / Tarim mixture and between 9 and 21% of ancestry from Lake Baikal. In addition, the ancient individuals of the Chemurchek culture have about two-thirds of the ancestry of the ancient individuals of Dzungaria and the rest from a mixture between Tarim / IAMC or BMAC.

The ancient individuals of Tarim are the result of a genetic mix between an ANE population (72%) and ancient individuals from the Lake Baikal region (28%). They do not have Afanasievo ancestry. The date of this genetic mixture is estimated at 183 generations before the date of these individuals, i.e. between 8000 and 6000 BC.

The body text of the paper explains:

Within and around the Dzungarian Basin, pastoralist Early Bronze Age (EBA) Afanasievo (3000–2600 BC) and Chemurchek (or Qiemu’erqieke) (2500–1700 BC) sites have been plausibly linked to the Afanasievo herders of the Altai–Sayan region in southern Siberia (3150–2750 BC), who in turn have close genetic ties with the Yamnaya (3500–2500 BC) of the Pontic–Caspian steppe located 3,000 km to the west. Linguists have hypothesized that the Afanasievo dispersal brought the now extinct Tocharian branch of the Indo-European language family eastwards, separating it from other Indo-European languages by the third or fourth millennium BC. However, although Afanasievo-related ancestry has been confirmed among Iron Age Dzungarian populations (around 200–400 BC), and Tocharian is recorded in Buddhist texts from the Tarim Basin dating to AD 500–1000, little is known about earlier Xinjiang populations and their possible genetic relationships with the Afanasievo or other groups.

The paper and its abstract are as follows:

The identity of the earliest inhabitants of Xinjiang, in the heart of Inner Asia, and the languages that they spoke have long been debated and remain contentious. Here we present genomic data from 5 individuals dating to around 3000–2800 BC from the Dzungarian Basin and 13 individuals dating to around 2100–1700 BC from the Tarim Basin, representing the earliest yet discovered human remains from North and South Xinjiang, respectively.
We find that the Early Bronze Age Dzungarian individuals exhibit a predominantly Afanasievo ancestry with an additional local contribution, and the Early–Middle Bronze Age Tarim individuals contain only a local ancestry. 
The Tarim individuals from the site of Xiaohe further exhibit strong evidence of milk proteins in their dental calculus, indicating a reliance on dairy pastoralism at the site since its founding. 
Our results do not support previous hypotheses for the origin of the Tarim mummies, who were argued to be Proto-Tocharian-speaking pastoralists descended from the Afanasievo or to have originated among the Bactria–Margiana Archaeological Complex or Inner Asian Mountain Corridor cultures. Instead, although Tocharian may have been plausibly introduced to the Dzungarian Basin by Afanasievo migrants during the Early Bronze Age, we find that the earliest Tarim Basin cultures appear to have arisen from a genetically isolated local population that adopted neighbouring pastoralist and agriculturalist practices, which allowed them to settle and thrive along the shifting riverine oases of the Taklamakan Desert.
Zhang, F., Ning, C., Scott, A. et al. "The genomic origins of the Bronze Age Tarim Basin mummies." Nature (October 27, 2021) (open access).

Horses Came Late In Indo-European Expansion

Another not fully paradigm supporting result derived from modern and ancient horse DNA is that while horses were sporadically domesticated on the steppe ca. 3500 BCE, only with the Sintashta culture ca. 2000 BCE did domesticated horses (and wheeled chariots) explode from the steppe in the the Middle East and Europe.
Domestication of horses fundamentally transformed long-range mobility and warfare. However, modern domesticated breeds do not descend from the earliest domestic horse lineage associated with archaeological evidence of bridling, milking and corralling at Botai, Central Asia around 3500 BC. Other longstanding candidate regions for horse domestication, such as Iberia and Anatolia, have also recently been challenged. Thus, the genetic, geographic and temporal origins of modern domestic horses have remained unknown. 
Here we pinpoint the Western Eurasian steppes, especially the lower Volga-Don region, as the homeland of modern domestic horses. Furthermore, we map the population changes accompanying domestication from 273 ancient horse genomes. This reveals that modern domestic horses ultimately replaced almost all other local populations as they expanded rapidly across Eurasia from about 2000 BC, synchronously with equestrian material culture, including Sintashta spoke-wheeled chariots. 
We find that equestrianism involved strong selection for critical locomotor and behavioural adaptations at the GSDMC and ZFPM1 genes. Our results reject the commonly held association between horseback riding and the massive expansion of Yamnaya steppe pastoralists into Europe around 3000 BC driving the spread of Indo-European languages. This contrasts with the scenario in Asia where Indo-Iranian languages, chariots and horses spread together, following the early second millennium BC Sintashta culture.
Pablo Librado, et al., "The origins and spread of domestic horses from the Western Eurasian steppes" 598 Nature 634–640 (October 20, 2021) (open access).

Thus, the early phases of Indo-European expansion into Europe by the Bell Beaker and Corded Ware cultures that preceded the Sintashta culture were not driven mostly by utilization of the domesticated horse, as previously believed, but by advantages including their Bronze age metallurgy and superior agricultural practices.

This is of a piece with the increasing realization that the Corded Ware people further to the north of the steppe zone, were from lightly forested regions rather than open plain, and the lack of a strong association between the Bell Beaker people and horse. Both groups, however, would have had cattle herding and may have had occasional horses even though the presence of these horses wasn't a dominant military factor until the Sintashta horse riding and chariot utilizing accoutrements were added to the package.

But, the horse driven Sintashta cavalry driven expansion may have been instrumental in Indo-European expansion into the Balkans, Greece and Anatolia, and into Iran and South Asia. This was also probably pivotal in the arrival of steppe admixture into the Near East although, south of the Hittite empire, it did not give rise to language shift to an Indo-European language.

Monday, February 22, 2021

Race, Legendary History, And Indo-Aryan Expansion

The Vedic epics are the oldest narrative stories of South Asia that survive, initially in reasonably accurate oral accounts in a milieu consistent with the Bronze Age that were eventually committed to writing. 

The Vedas, like the Bible and the Scandinavian epic poems, are a composite of different works composed at different times, with the oldest works in particular constituting "legendary history", which draw on factual history reality and purely fictional myths of cultural relevance in an undifferentiated whole. 

Legendary history is particularly common globally in Bronze Age cultures, and continues into the early Iron Age, with newly composed works retreating in the later Classical era, but enjoying a resurgence after the fall of Rome, with the Medieval European "Lives Of Saints" genre and some accounts of the Crusades, constituting its last hurrah, before reliable secular history and myth become fully divorced from each other again. There are probably reasons for this reality rooted in the economic and technological limitations of these eras.

Discerning what portion of legendary history is myth and what portion reflects historical reality is more art than science and requires resort to sources beyond these texts to resolve satisfactorily. But archaeology, linguistics and genetics (especially ancient DNA techniques) have started to pave the way to clarify these points, as, for example, in the case of the Illiad and related works which are a legendary history of Trojan War on the Aegean coast of what is now the country of Turkey in the decades leading up to Bronze Age collapse.

His post tends to corroborate the concept expressed in my previous post today about Neolithic expansion in Europe and the subsequent marginalization of the first farmers of Europe (just like the marginalization of European hunter-gathers by the first farmers) that the population genetic communities that emerged from these clashes of civilizations was strongly influenced by racism.

Razib Khan notes at Brown Pundits, and I agree (including regarding the time and place that the Vedas were composed and its likely sources) that:
The Indo-Aryans described the natives of the subcontinent as dark and “snub-nosed.” That their arrival in some ways was a meeting of two different races.
3,000-4,000 years ago a people who resembled what we would term “white” expanded within the Indian subcontinent. If modern Armenians are white, then the Indo-Aryans were white. At least initially. In the subcontinent, they met a variety of people. Some of them, such as in Sindh, were of brownish complexion. Others, to the south and east, would have been considerably darker. I also assume that the Vedas were constructed in situ in the Indian subcontinent. That is, they reflect a milieu of people who were encountering the northwest of the subcontinent, and had recently traversed through BMAC (Indra may actually be a BMAC diety).

What’s the upshot here? I now think that the metaphorical view of the physical descriptions should be set next to the literal view. The reality is probably a mix. But the fact is that groups with very different physical appearances did interact in ancient India. The Aryans were almost certainly very light-skinned, with “sharp features”, in comparison to many of the people they encountered. Though one can construct hybrid scenarios, where Indo-Aryan enemies were described in inaccurate ways precisely because those tropes were associated with tribes and peoples the Indo-Aryans had conquered.

Better Ancient DNA Analysis Sheds LIght On European Neolithic Dispersion

The Short Version

Improved analysis of rare types of ancient Y-DNA from the Neolithic era in Europe confirms that there were two genetically distinct populations that brought farming with them in a mass migration replacing prior European hunter-gatherers in Europe, one by a Danubian route associated with the LBK culture, and one by a Northern Mediterranean route associated with the CP culture.

The analysis also provides a good example of more general processes in how the populations genetics of a large region changes in a punctuated manner driven by cultural divisions between genetically distinct groups (in this case, basically, by racism of the steppe people directed towards Europe's first farmers).

The Long Version

A new method called YMCA allows for more precise characterization of Y-DNA found in ancient DNA samples. 

This has been used to reanalyze the rare (in Europe) Y-DNA H2 samples from the Neolithic era to shed more light on how farmers dispersed through Europe, supporting the archaeologically supported hypothesis that the expansion involved a distinct Daunbian Linear Pottery (LBK) culture and a Northern Mediterranean Cardial Pottery (CP) culture. Each migration group was a genetically distinct population that contained a small number of individuals with distinct rare Y-DNA H2 haplotypes that serve as markers of distinct populations following each route.

The following quotes are from a Google translation of a recent post at Bernard's Blog (the original is in French) discussing a new paper by Rochrlach, et al. at bioRxiv:

Haplogroup H is believed to have emerged in South Asia around 48,000 years ago. Its three branches H1-M69, H2-P96 and H3-Z5857 then appeared rapidly between 44,000 and 45,000 years ago. H1 and H3 are found today at frequencies of up to 20% in South Asia, but at very low frequency in Europe.  

In particular H1 is associated with the arrival of Roma populations about 900 years ago.  

The H2 branch has been present in Europe for much longer since it arrives with the first farmers of the Neolithic. It is thus found at frequencies of 1.5 to 9% depending on the archaeological sites. Today, however, it is present at frequencies below 0.2% in Europe.

The authors therefore applied the new YMCA method to 58 European Neolithic haplogroup H2 samples. Until now the H2 haplogroup has been divided into three sub-branches: H2a, H2b and H2c obtained from contemporary genomes.  

Analysis of the ancient genomes of the European Neolithic revealed two new sub-branches: H2d and H2m both further divided into two sub-branches: H2d1, H2d2, H2m1 and H2m2. . . .

Interestingly all H2d haplogroup samples are located on the Danubian route of the European Neolithic, while all H2m haplogroup samples are located on the Mediterranean route, all the way to the Iberian Peninsula and beyond into Ireland. A sample threshold H2m is found in Central Germany, but it is dated to the end of the Neolithic.

The authors then dated the common ancestor of the H2 branch to approximately 24,100 years, the H2d and H2m sub-branches to approximately 15,400 years, the H2m1 and H2m2 sub-branches to approximately 13,300 years and the H2d1 and H2d2 sub-branches to about 11,900 years old.

The dates at which the subclades emerged are in the Mesolithic era, appropriately prior to the Fertile Crescent Neolithic revolution and its expansion into Europe around 8,000 years ago.

The fairly high, although minority percentage of Y-DNA H in the first farmer wave of Europe is also a notable fact in and of itself that would not obviously be suspected and does not have a full explanation.

Why Did Y-DNA H Decline In Frequency So Dramatically?

The decay in the fraction of Y-DNA H in Europe is partially due to direct decline by dilution from the expansion of steppe people with horses and metal into Europe in the late Neolithic and early Bronze Age. But more than simple dilution was at work. 

Y-DNA haplogroups are particularly prone to changes in frequency in societies organized on a patrilineal basis when one culture displaces another in a leadership role. 

This is in part because men of the defeated culture are massacred. 

It is in part, because men of the defeated culture have a harder time obtaining wives. 

And, it is in part, because men of the defeated culture are deprived on a relative basis of resources like food. Malnutrition reduces the chances their children have of survival not only directly from starvation. It also reduces their chance of survival indirectly due to their children's increased vulnerability to disease, and their wives' vulnerability to miscarriage and stillbirth, when malnourished.

Also, not all Neolithic Y-DNA groups declined in the same proportion. This is because lower frequency Y-DNA haplogroups in a population are disproportionately lost in a period of declining frequency, such as the experienced by men with patrilineal descent from the first farmers of Europe rather than from subsequent steppe people, relative to higher frequency Y-DNA haplogroups. 

Thursday, December 31, 2020

An Overview Of East Asian and Southeast Asian Historical Linguistics

Overview

There are nine main language families in Southeast Asia and East Asia: Japonic (Japanese and a couple of related languages spoken on remote Japanese languages), Korean, Ainu (a language isolate spoken by indigenous people of Northern Japan), Sino-Tibetan (including Chinese, the Tibetan languages and Burmese), Austronesian (also spoken in Polynesia), Thai-Kadai a.k.a. Kra-Dai (of which the language of Thailand is best known), Austroasiatic a.k.a. Mon-Khmer (the most famous of which are Vietnamese and the Munda languages of India and also including the Khmer languages of Cambodia) and Hmong-Mien (a language family of an important minority population in Southeast Asia and South China). 

Genetic and linguistic evidence, however, shows that the Hmong-Mien language family is an offshoot of the Austroasiatic language family. There is strong but not universally accepted evidence that Austroasiatic languages and Thai-Kadai languages are part of a larger macro-language family. There is strong but not universally accepted evidence that the Japonic and Korean languages are part of the same language family.

Sino-Tibetan languages have their roots in the North Chinese millet farming Neolithic revolution on the Yellow River. 

The other four language families have their roots in the Southern Chinese rice farming Neolithic revolution on the Yangtze River. The Austronesian and possibly the Thai-Kadai language families originate in the lower Yangtze River basin. The Austroasiatic, Hmong-Mien and possibly the Thai-Kadai language families originate in the middle Yangtze River basin.

It is likely that none of the major languages of Southeast Asia were spoken there prior to about 2200 BCE. Prior to that point, Southeast Asia was largely populated by Hoabinhian hunter-gatherer populations whose languages are largely lost.

Y-DNA evidence suggests that Austronesian language family speakers are an out group to the other four major Southeast Asian and East Asian language families (Sino-Tibetan, Austroasiatic, Hmong-Mien, Thai-Kadai), with people speaking those languages linked to Austronesians only at a greater time depth.[1] This could be a misleading signal driven by the admixture of Austronesians with Austro-Melanesian populations, however.

The World In 4100 BCE

In 4100 BCE, domesticated rice was not available anywhere in the world except (1) the Yangtze River basin and (2) in the Ganges River basin in India (where it was just a few hundred years old as a domesticated crop). It would be domesticated in South American about a century after that. 

At that time, domesticated millet was not available anywhere in South Asia, Southeast Asia or East Asia except in the Yellow River basin and its near vicinity.

The World In 3100 BCE 

In 3100 BCE, farming was absent, and Paleolithic hunter-gatherers were the sole inhabitants of Japan, Taiwan, mainland Southeast Asia, island Southeast Asia, Papuan New Guinea and the immediately adjacent islands, the Philippines, Australia, and all of South Asia to the east of the Indus river Valley, the now barren Sarasvati river basin and the Ganges river basin. 

None of the languages spoken in Southeast Asia (other than the Papuan languages) or Taiwan or the Philippines today were spoken there. The only language now spoken in in the Japanese islands that existed then was Ainu.

None of the languages now spoken in South Asia or Iran today were spoken there, with the possible exception of the Dravidian languages. The Dravidian languages, if spoken at all, were confined to the small tribes of hunter-gatherers who would adopt farming for the first time in Southern India in the South Indian Neolithic Revolution. 

Oceania from Hawaii and Easter Island to Guam and the Mariana Islands to Fiji and Tonga and the Cook Islands and New Zealand, and also Antarctica, were places where no primate, let alone a modern human, had ever set foot.

In Africa, Bantu expansion had not yet begun, so pretty much all of Africa to the South of the Congo River basin and the jungles of the Congo, and much of East Africa, was inhabited only by hunter-gatherers, and racial and linguistic diversity in Africa was much greater. Likewise, the ethnogenesis of the Berber people had not yet occurred.

In Europe, people with the new predominant Northern European phenotypes (e.g. people with blond hair and blue eyes) did not exist and Indo-European languages were confined to Eastern Europe. The percentage of ancestry of modern Irish people traceable to 3100 BCE is close to negligible as it underwent near total population replacement.

The Ainu Language

The Ainu language is derived from one of the languages of the Jomon hunter-gathers of Japan who inhabited the area from the paleolithic era. It was probably influenced by or related to Paleo-Siberian languages. All of these languages are now nearly moribund.

The Japonic and Korean Languages

The Japanese languages arose when the Yayoi people migrated to Japan from Korea ca. 400 BCE to 300 BCE, derived from the pre-existing language, probably a sister language to Korean, spoken by these people. The deep origins of the Korean language in pre-history aren't well understood.

The Austronesian Languages

The Austronesian expansion from Taiwan began about 3000 BCE, and this expansion of one of the indigenous languages of Formosa is arguably really what defines this language family.[2] The indigenous Formosan languages are probably all derived from the Neolithic Dapenkeng culture that abruptly appeared and quickly spread around the coast of the island around 4000 BCE to 3000 BCE (displacing prior Negrito hunter-gatherer populations), only preceding the migration of one of those cultures to other islands by within the margin of error of available dating methods.[3] The particular archeological culture of mainland South China from which this culture was derived is unresolved, in part because archaeological data from that time period is sparse and undeveloped.[4] 

The Sino-Tibetan Languages
[T]he main ancestry of high-altitude Tibeto-Burman speakers originated from the ancestors of Houli/Yangshao/Longshan ancients in the middle and lower Yellow River basin, consistent with the common North-China origin of Sino-Tibetan language and dispersal pattern of millet farmers.[5]
This conclusion is contrary to many 20th century and early 21st century proposals (putting a homeland in Northeast India or Southern China) but now probably represents conventional wisdom in the field.[5]

So, the Sino-Tibetan languages date the North Chinese Neolithic Revolution which was millet farming and independent in origin from South Chinese and Southeast Asian rice farming. The earliest archaeological culture in this region is the Nanzhuangtou culture which started around 8500 BCE, but it isn't clear that that culture was in linguistic continuity with the cultures that gave rise to the Sino-Tibetan language family. Two major studies in 2019 favor this model but assign a more recent origin to the language family than the first Neolithic culture of the region:
Zhang et al. (2019) performed a computational phylogenetic analysis of 109 Sino-Tibetan languages to suggest a Sino-Tibetan homeland in northern China near the Yellow River basin. The study further suggests that there was an initial major split between the Sinitic languages and the Tibeto-Burman languages approximately 4,200 to 7,800 years ago [2200 BCE to 5800 BCE] (with an average of 5,900 years ago [3900 BCE]), associating this expansion with the Yangshao culture and/or the later Majiayao culture. Sagart et al. (2019) also performed another phylogenetic analysis based on different data and methods to arrive at the same conclusions with respect to the homeland and divergence model, but proposed an earlier root age of approximately 7,200 years ago [5200 BCE], associating its origin with the late Cishan and early Yangshao culture.[6]
The Northern millet farmers and Southern Rice farmers started to integrate into a common culture in which the Han Chinese component eventually became dominant around 3500 BCE.[7]

Other Southeast And East Asian Language Families

Rice was domesticated in Southern China around 7400 BCE.[8] But that doesn't mean that the initial rice domesticating culture was in linguistic continuity with the first Austro-Asiatic populations. And the time depth of the various language of the region is muddy. 
There are two most likely centers of domestication for rice as well as the development of the wetland agriculture technology. 
The first, and most likely, is in the lower Yangtze River, believed to be the homelands of the pre-Austronesians and possibly also the Kra-Dai, and associated with the Kauhuqiao, Hemudu, Majiabang, Songze, Liangzhu, and Maqiao cultures. It is characterized by pre-Austronesian features, including stilt houses, jade carving, and boat technologies. Their diet were also supplemented by acorns, water chestnuts, foxnuts, and pig domestication.

The second is in the middle Yangtze River, believed to be the homelands of the early Hmong-Mien-speakers and associated with the Pengtoushan, Nanmuyuan, Liulinxi, Daxi, Qujialing, and Shijiahe cultures. Both of these regions were heavily populated and had regular trade contacts with each other, as well as with early Austroasiatic speakers to the west, and early Kra-Dai speakers to the south, facilitating the spread of rice cultivation throughout southern China.

By the late Neolithic (3500 to 2500 BC), population in the rice cultivating centers had increased rapidly, centered around the Qujialing-Shijiahe culture and the Liangzhu culture. Liangzhu and Shijiahe declined abruptly in the terminal Neolithic (2500 to 2000 BC). With Shijiahe shrinking in size, and Liangzhu disappearing altogether. This is largely believed to be the result of the southward expansion of the early Sino-Tibetan Longshan culture. ... This period also coincides with the southward movement of rice-farming cultures to the Lingnan and Fujian regions, as well as the southward migrations of the Austronesian, Kra-Dai, and Austroasiatic-speaking peoples to Mainland Southeast Asia and Island Southeast Asia. A genomic study also indicates that at around this time, a global cooling event (the 4.2 k event) led to tropical japonica rice being pushed southwards, as well as the evolution of temperate japonica rice that could grow in more northern latitudes.[7]  
The Tai-Kadai Languages

The Tai-Kadai languages are now most widely spoken in the mainland Southeast Asian country of Thailand, but, this is actually the most recent language family to arrive in Southeast Asia from Southern China.
The high diversity of Kra–Dai languages in Southern China points to the origin of the Kra–Dai language family in Southern China. The Tai branch moved south into Southeast Asia only around 1000 CE.[9]
Genetically, the biggest difference between the Tai-Kadai people within Southeast Asia, and the Austroasiatic populations of Southeast Asia, both of whom have origins in the early Neolithic rice farmers of the Yangtze River basin of Southern China, is that Austroasiatic people, having arrived earlier, have more Hoabinhian hunter-gatherer admixture.[10]

There is strong, but not universally accepted evidence that the Thai-Kadai language family and the Austronesian language family are part of a larger macro-language family.[11]

The Austro-Asiatic and Hmong-Mien Languages

The Austroasiatic language family is probably derived from Southern Chinas Neolithic Rice farmers who trace their culture origins to the domestication of Chinese rice in an independent domestication event. Ancient DNA suggests that this is was the first of the language families of modern Southeast Asia to be spoken there by people who resided there.

The expansion from South China to Southeast Asia took place around 4,000 years ago and close in time to the spread of the Austronesians in Southeast Asia. They displaced Hoabinhian hunter-gatherer populations in Southeast Asia.[12] 

Ancient DNA shows populations genetically similar to modern Austro-Asiatic populations in Vietnam, Laos, and mainland Malaysia by 2200 BCE. [13] But the archaeological record is thin in the relevant time period from the South Chinese Neolithic revolution to 2200 BCE, so dating it is tricky. Still, the oldest ancient DNA may have been from close to the time that the language family arrived there since:
The spread of japonica rice cultivation to Southeast Asia started with the migrations of the Austronesian Dapenkeng culture into Taiwan between 3500 and 2000 BC (5,500 BP to 4,000 BP). The Nanguanli site in Taiwan, dated to ca. 2800 BC, has yielded numerous carbonized remains of both rice and millet in waterlogged conditions, indicating intensive wetland rice cultivation and dryland millet cultivation. A multidisciplinary study using rice genome sequences indicate that tropical japonica rice was pushed southwards from China after a global cooling event (the 4.2k event) that occurred approximately 4,200 years ago.[13] 

A genetically based conclusion that the Hmong-Mien peoples are a comparatively recent offshoot of the Mon-Khmer peoples, something that linguistic analysis has not reached consensus upon, is a finding of considerable importance in parsing out the prehistory of Southeast Asia, even though the hypothesis that Mon-Khmer and Hmong-Mien both belong to a macrolinguistic family (sometimes called Yangtzean) has existed for some time as one of several efforts to link the languages of South China and Southeast Asia into linguistic macrofamilies. An expanded study of Y-DNA population genetics in Southeast Asia by Chinese researchers, confirms that close genetic ties of Mon-Khmer (a.k.a. Austro-Asiatic when the Munda of India are also included) and Hmong-Mien peoples, at least in the patriline, focusing on the O3a3b-M7 Y-DNA haplogroup where the Mon-Khmer appearing at a basal position while Hmong-Mien and Tibeto-Burmese individuals with this hapologroup have subhaplogroups more on the fringes of this patriline tree. O3a3c1-M117, the dominant East Asian haplogroup shows a similar pattern.[1] 

References 

[1] Cai X, et al. "Human Migration through Bottlenecks from Southeast Asia into East Asia during Last Glacial Maximum Revealed by Y Chromosomes." PLoS ONE 6(8): e24282 (2011). doi:10.1371/journal.pone.0024282 


[3] Wikipedia article on History of Taiwan: Early settlement. 


[6] Wikipedia article on Sino-Tibetan languages: Homeland citing Zhang, Menghan; Yan, Shi; Pan, Wuyun; Jin, Li (2019), "Phylogenetic evidence for Sino-Tibetan origin in northern China in the Late Neolithic", Nature, 569 (7754): 112–115, and Sagart, Laurent; Jacques, Guillaume; Lai, Yunfan; Ryder, Robin; Thouzeau, Valentin; Greenhill, Simon J.; List, Johann-Mattis (2019), "Dated language phylogenies shed light on the history of Sino-Tibetan", Proceedings of the National Academy of Sciences of the United States of America, 116 (21): 10317–10322.

[7] Wikipedia article on Rice: Origins in China


[9] Wikipedia article on Kra-Dai languages


[11] Wikipedia article on Austro-Tai languages.


[13] Wikipedia article on Rice: Southeast Asia

Sunday, December 27, 2020

What Will Humans Look Like In 100,000 Years

A cute little speculative article imagines what humans might look like 100,000 years from now due to evolution after living in space for a while with a before and after picture.

Now


In 100,000 years

The article motivates its pictures as follows: 

In 2007, artist and researcher Nickolay Lamm partnered with computational geneticist Dr. Alan Kwan and came up with three illustrations. He first hypothesized what we might look like in twenty thousand years, the second in sixty thousand years, and the third 100 thousand years into the future.

According to Lamm, this is “one possible timeline” that takes into consideration both human evolution and advancements in technology and genetic engineering. Lamm and Kwan imagined a possible future where humans would have a much greater ability to control the human genome, and where their living environments might be much different than ours [1].

Here are some of the major changes that could happen, and the reasons why they might occur, according to Kwan and Lamm: 
A larger forehead 

The human forehead has been increasing in size since the fourteenth and fifteenth centuries. According to scientists, when you measure skulls from that time and compare them to our own, people today have less prominent facial features and higher foreheads [2]. It seems logical, then, to imagine a future where our skulls continue to grow to accommodate larger and larger brains. 
Changed Facial Features

Given the advancements we have already made in genetic engineering, Kwan based some of his hypotheses on the assumption that we will be even further ahead sixty thousand years from now. He argued that a greater ability to control the human genome will mean that evolution will have little effect on human facial features. Essentially, our faces will change depending on human preferences- like larger eyes, a straighter nose, and more symmetry between both sides of our faces. 
He also suggested that by then, it is possible that humans will have begun colonizing other planets. People living in places that are further from the sun, and therefore are less bright, may cause their eyes to get bigger to enhance vision. Skin may also be darker to lessen the damage from UV rays outside of earth’s protective atmosphere.
Additionally, he proposed that people will have thicker eyelids, and their frontal bone under their brow will be more pronounced. This will help humans to deal with the disruptive effects of cosmic rays. We already see these effects happening with today’s astronauts.

Kwan says that over the remaining forty thousand years, those features that humans selected for will become even more pronounced. One hundred thousand years from now, it is possible that humans’ eyes, for example, will seem unnervingly large compared to what we are used to today. 
Functional Necessities

Other, smaller changes may be things like larger nostrils. This will allow humans to breathe easier when they’re living on other planets. People may have denser hair to keep their larger heads warm. In an age, however, when you can genetically alter almost any feature about yourself, Kwan suggests that features make us look naturally human will become more favorable.

It is an interesting exercise although it misses some obvious points.

Time Horizons

The notion that this would happen over 100,000 years based upon past experience of the human species is not very credible for the kind of basic visual phenotypes focused upon.

Most of the common phenotypes associated with major "racial" types today evolved much more rapidly. There was no one in Europe who looked like a typical modern Northern European in 4000 BCE. 

Bantu expansion in Africa, in the same time period, caused one West African phenotype to become predominant in most of sub-Saharan Africa, leaving only small relict populations of "Paleo-Africans" like pygmies and Khoi-San people, and subtly reducing the distinctiveness of the typical linguistically Nilo-Saharan East African.

A lot of the distinctiveness of East Asian phenotypes is attributable to the selective sweep of the EDAR gene which is much older than either of the other two examples, but happened, when it did happen, in a matter of a few thousand years, not tens or hundreds of thousands of years.

Genetic engineering, to the extent it occurs, will likewise have its biggest impacts in a matter of a century or two, not thousands of years. And, while the article notes that some geneticists at the time put the prospects of this kind of genetic engineering thousands of years in future, CRISPER technology already available and still in its infancy with lots of room to improve, suggests that this is much less far off than expected in 2007 when it was done, especially for visually striking, but largely cosmetic features that involve only small numbers of genes like eye, hair and skin color, hair texture and curliness, propensity to tan, and freckles.

Genetic engineering will probably start with efforts to actively select against "defects" from Downs' syndrome to bad teeth and vulnerability to specific genetic diseases with simple recessive Mendelian inheritance patterns. Simple cosmetic adjustments that are well understood may follow. And, from there, the chase for enhancements, such as additional cones that allow people to see more colors, may begin. I see those steps taking perhaps a generation or two at a time to progress from one level to the next.

I fully expect the appearance of the average human to be significantly visually different by 3000 CE, not merely tens of thousands of years hence.

Admixture

Sufficiently far in the future, there will be few, if any, people who are phenotypically comparable to modern Europeans, due to admixture.

The world almost surely will see dramatically more admixture over the next few centuries than it has since the Bronze Age. In this regard Betty Crocker has probably been more predictive in forming a composite, mixed race, customer of the company:

For her 75th anniversary in 1996, a nationwide search found 75 women of diverse backgrounds and ages who embody the characteristics of Betty Crocker. The characteristics that make up the spirit of Betty Crocker are: enjoys cooking and baking; committed to family and friends; resourceful and creative in handling everyday tasks; and involved in her community. A computerized composite of the 75 women, along with the 1986 portrait of Betty, served as inspiration for the painting by internationally known artist John Stuart Ingle. The portrait was unveiled March 19, 1996, in New York City.

Better yet is this National Geographic image:

Selection On Standing Variation


Image from here.

The massive intercontinental admixture we are likely to see also reflects another key point of both natural evolution and selective breeding, which is that most evolutionary selection involves selection within the existing range of variation among people, rather than new mutations that prove beneficial, which are the exception.

Indeed, one of the real challenges in the first wave of genetic engineering will be to avoid the temptation to completely remove genetic diversity, biodiversity and neurodiversity from the human species when it seems to be a net minus in current conditions from the standing range of variation in humans only to discover that these traits may have currently unrecognized benefits sometime long in the future. Otherwise, the demise of human genetic diversity could mirror the mass extinction of species and languages on Earth during the late Holocene. 

Lots of the most important bits, like HLA immunity complexes and temperaments better suited to the world of the far future, are also largely invisible a priori although their functional connection to other traits may make that less true than one would expect as discussed below.

On the other hand, genetic engineering can revolutionize that analysis. For example, if we find a gene that is very valuable in extremely genetically dissimilar octopi that is total absent from vertebrate genetic diversity a few decades from now, we might very well use genetic engineering to make that a common variant in the human genome.

Self-Domestication

Humans are likely to continue to select for traits associated with domestication of animals, a process that is already well underway.
Darwin observed that domesticated animals share certain traits across species. Domesticates tend to have floppier ears than their wild counterparts, and curlier tails. They're smaller and have recessed jaws and littler teeth. Domestication also shrinks the amygdala, the brain's fear center, leading to a reduction in aggressive, fearful reactions.

Belyaev noticed that his domesticated foxes eventually developed black and white, or piebald, spots, now known to be a classic sign of domestication. Think of the black and white pelts of cows, horses, dogs, and cats – especially those white-footed felines we claim "wear socks."

The thing is, with the exception of docility, these characteristics don't do anything at all.

Research like Belyaev's made it apparent that if you select for friendliness and cooperation in foxes, you get a host of features that come along for the ride that don't serve a purpose – in evolutionary parlance they're non-adaptive, much like the male nipple. Together this suite of traits is called the "domestication syndrome."

For years scientists have recognized that domestication seems to preserve childlike psychological and physical tendencies, especially those that elicit care from parents and other adults. "Cuter" features. A little more helplessness. And friendliness towards humans, supporting Hare's argument. Recent science has helped piece together why this is.

During vertebrate development there is a strip of what are called neural crest cells running down the back of the embryo. As we grow inside the womb, these cells migrate throughout the body to help form the cartilage and bone of our face and jaw, the melanin-producing cells that give our skin pigment, and part of our peripheral nervous system. They also form our adrenal glands, which, among other functions, release cortisol — our "stress hormone" — and adrenaline, involved in our fight or flight response.

Domesticated animals have smaller adrenal glands. Hare believes selection for friendliness results in less neural crest migration, and as a result, less aggressive, reactionary behavior driven by adrenal hormones.

But fewer neural crest cells reaching their intended targets also influences the other traits driven by their voyage through the body, explaining the smaller snouts and jaws seen in domesticates, and white patches of fur lacking melanin. Scientists now know that domestication — whether artificial or natural — seems to involve selection on a gene called BAZ1B, which helps drive neural crest migration during development.
Baby faces are the future. Other related traits, like enhanced childhood language learning relative to adults, may also be the subject to genetic engineering in the future. William's Syndrome illustrates what this might look like, which bears some similarities to mythical elves:


Technology Facilitates Adaptation And Determines What Is Selected For

Technology can also reduce selective pressure on a lot of obvious physical features, like skin color, with things like Vitamin D supplements and sun screen picking up the slack.

Technology can also determine which human traits merit selection.

For example, for most of human history, food supplies with limited and irregular, and there was strong selection for a capacity to survive periods of famine. But in the modern world, selection is likely to focus on an ability to escape the downsides of obesity that present themselves in a more sedentary world where food is abundant and consistently available.

Physically wild movement and hyperactivity may have been beneficial in much of human history, while the future looks likely to reward a capacity to be still and focused.

Some traits may be the subject to genetic engineering, while other forms of non-genetic bioengineering like nutritional supplements, vaccines, and hormone treatments may also play important parts. Nutrition without genetics can prevent common visible consequences of malnutrition and can enhance height. Everyone in the future will probably be more health overall based upon a variety of genetic and non-genetic methods and cultural adaptations to modern technologies that we are struggling with now.

We might end up with genetic engineering that mitigates nearsightedness adapting to a world where reading fine print regularly is essentially, but if laser eye surgery continues to advance, that may not be a priority as other forms of bioengineering will do the trick.

Self-driving cars and other intelligent safety features in mechanical and chemical things may reduce the selective effects that our current society has against people who impulsively drive too recklessly, cross the street without carefully looking both ways, drink and drive, or otherwise engage in conduct that has grown much more deadly for the average persons than it did in the days where land travel was mostly by foot. Likewise, vulnerability to jet lag might be less important in an era of self-driving cars and AI safety features, when grogginess can be deadly, than in one without them.

Intelligence has lots of value in the modern world, but large infant head size also increases the risk of death to mother and child in natural child birth. But this risk may be alleviated in C-sections are universally and widely available, allowing for larger heads and bigger brains (even though average brain size seems to be declining in recent decades).

Another factor that has impeded brain size development is energy drain. The brain uses 20% of the body's energy demand while only 4% of its volume. But if more energy efficient neurons were genetically engineered somehow, that might make it more workable to have larger brains without the metabolic cost faced by prior vertebrates.

At some point, we might want to genetically engineer humans to have natural immunity to lots of diseases, but in the meantime, improved vaccines might make that a low priority.

The interactions of technology and selective pressures make what the future of humanity looks like difficult to predict. A hundred thousand years out, who knows? Maybe we'll look like this:
Thursday, November 12, 2020

Explaining The Genetic Fitness Advantage Of LP and EDAR and Skin Color

In West Eurasia, the strongest target of genetic selective fitness adaptation is lactase persistence (LP) (see also here) which allows adults to drink milk, which surged around the time that Indo-Europeans migrated en masse across Europe in the late Neolithic era and early Bronze Age (often were more herding based food production than the first wave Neolithic populations of Europe derived from Anatolian farmers), and with sometimes regionally distinct genes that have the same effect, upon the arrival of pastoralism in the Near East and Africa.

In East Eurasia and the Americas, the EDAR gene which is responsible for much of the distinctively "East Asian" phenotype is a similarly powerful selective fitness adaptation in the Upper Paleolithic era (roughly speaking, after humans expanded out of Africa and before agriculture was developed). What specifically does it do?
A derived G-allele point mutation (SNP) with pleiotropic effects in EDAR, 370A or rs3827760, found in most modern East Asians and Native Americans but not common in African or European populations, is thought to be one of the key genes responsible for a number of differences between these populations, including the thicker hair, more numerous sweat glands, smaller breasts, and the Sinodont dentition (so-called shovel incisors) characteristic of East Asians. This mutation is also implicated in ear morphology differences and reduced chin protrusion. 
The mutation arose in humans approximately 30,000 years ago, and now is found in 93% of Han Chinese and in the majority of people in nearby Asian populations. 
It has been hypothesized that natural selection favored this allele during the last ice age in a population of people living in isolation in Beringia, as it may play a role in the synthesis of breast milk under Vitamin D-poor conditions. 
Previous research has shown that both LP and EDAR genes may make it easier for mothers to get Vitamin D and/or to pass Vitamin D to their children during pregnancy and in breast feeding. 

But, what is so great about mothers having high levels of Vitamin D and passing it on to their children?

Well, it turns out that the presence of Vitamin D in a mother during pregnancy enhances the IQ of her children, which has great potential to be fitness enhancing, on top of benefits like preventing miscarriage, enhancing fertility, and having immune system enhancing properties.

The importance of Vitamin D could also explain apparent selective fitness effects of matching skin color appropriately to latitude, i.e. favoring pale skin at high latitudes to enhance Vitamin D levels, while favoring darker skin at lower latitudes where solar exposure is more intense to prevent sun burns and skin cancer where it is possible to get sufficient Vitamin D even with darker skin.

The paper and its abstract are as follows:
Background

Vitamin D is critical to embryonic neuronal differentiation and other developmental processes that may affect future neurocognitive function. However, observational studies have found inconsistent associations between gestational vitamin D and neurocognitive outcomes. 
Objectives

We examined the association of gestational 25-hydroxyvitamin D [25(OH)D] with children's IQ at 4–6 y, and explored whether associations differed by race. 
Methods

This study used data from the CANDLE (Conditions Affecting Neurocognitive Development and Learning in Early Childhood) cohort. Between 2006 and 2011, CANDLE recruited 1503 women in their second trimester of healthy singleton pregnancies. Inclusion criteria for this analysis were gestation of ≥34 wk and availability of 25(OH)D and IQ data. Associations between second-trimester 25(OH)D plasma concentration and Stanford-Binet IQ scores in offspring at 4–6 y were examined using multivariable linear regression; interaction terms were used to explore possible effect modification by race. 
Results

Mean ± SD 25(OH)D concentration among 1019 eligible dyads was 21.6 ± 8.4 ng/mL, measured at a mean ± SD gestational age of 23.0 ± 3.0 wk. Vitamin D deficiency [25(OH)D < 20 ng/mL] was observed in 45.6%. Maternal 25(OH)D differed by race with a mean ± SD of 19.8 ± 7.2 ng/mL in Blacks sand 25.9 ± 9.3 ng/mL in Whites ( P < 0.001). In adjusted models a 10-ng/mL increase in 25(OH)D was associated with a 1.17-point higher Full Scale IQ (95% CI: 0.27, 2.06 points), a 1.17-point higher Verbal IQ (95% CI: 0.19, 2.15 points), and a 1.03-point higher Nonverbal IQ (95% CI: 0.10, 1.95 points). We observed no evidence of effect modification by race. 
Conclusions

Second-trimester maternal 25(OH)D was positively associated with IQ at 4–6 y, suggesting that gestational vitamin D status may be an important predictor of neurocognitive development. These findings may help inform prenatal nutrition recommendations and may be especially relevant for Black and other dark-skinned women at high risk of vitamin D deficiency.
Melissa M Melough, et al., "Maternal Plasma 25-Hydroxyvitamin D during Gestation Is Positively Associated with Neurocognitive Development in Offspring at Age 4–6 Years." The Journal of Nutrition (2020). DOI: 10.1093/jn/nxaa309